Some fossils transcend the significance of a single species and become symbols of entire scientific ideas. Archaeopteryx is one of them.
Ever since the first specimens were discovered in the German limestone formations of Solnhofen in the nineteenth century, this unusual animal — with feathers and wings, but at the same time also with teeth, a long bony tail, and claws on its forelimbs — has become an almost textbook illustration of the evolutionary transition between theropod dinosaurs and birds.
For generations of students, it was presented as one of the most famous “missing links.” Today we know that the metaphor of a link is itself too simple. Evolution is not a chain in which one missing piece has to be found, but rather a branching network in which different lineages test different solutions, some survive, others disappear, and certain evolutionary innovations arise more than once and in different combinations.
For that reason, Archaeopteryx has not become less important. Quite the opposite. After more than 160 years of research, new techniques are beginning to extract information from its fossils that researchers of the nineteenth and twentieth centuries could not even see.
The fossil has not changed. What has changed is what we are capable of reading from it.
An Icon of Evolution from an Unusual Lagoon
Archaeopteryx lived about 150 million years ago, during the Late Jurassic, in what is now Bavaria. Bavaria at that time, of course, looked nothing like modern Central Europe. Solnhofen was an archipelago of low islands, lagoons, and shallow seas in a warm and predominantly dry climate. More recent reviews of its ecology describe a semi-arid, seasonally humid environment with vegetation probably dominated by low conifers, cycads, and ferns.
The special conditions in the lagoons made exceptional preservation possible. Fine-grained carbonate sediment, highly unfavorable conditions for life on the bottom, and rapid burial preserved details that disappear in most other fossil sites. Thanks to that, we can even recognize feather impressions today.
But here too, the story is no longer as simple as it once seemed. Only a small number of exceptionally important avialan fossils are known from Solnhofen, and most of them have at one time or another been assigned to the genus Archaeopteryx. Modern analyses show that there is still no complete consensus about their exact taxonomic relationships. It is possible that not all specimens represent a single species, or perhaps even a single early avialan lineage.
That is an important lesson: even one of the most famous fossils in the history of biology is not an “archived story” that no longer needs to be reopened.
When an Old Fossil Is Examined with a New Technique
When the first Archaeopteryx specimens were discovered, researchers had the naked eye, a magnifying glass, a microscope, and the chemistry of their time. Today we have computed tomography, digital image processing, chemical mapping, and one particularly interesting technique: laser-stimulated fluorescence, LSF.
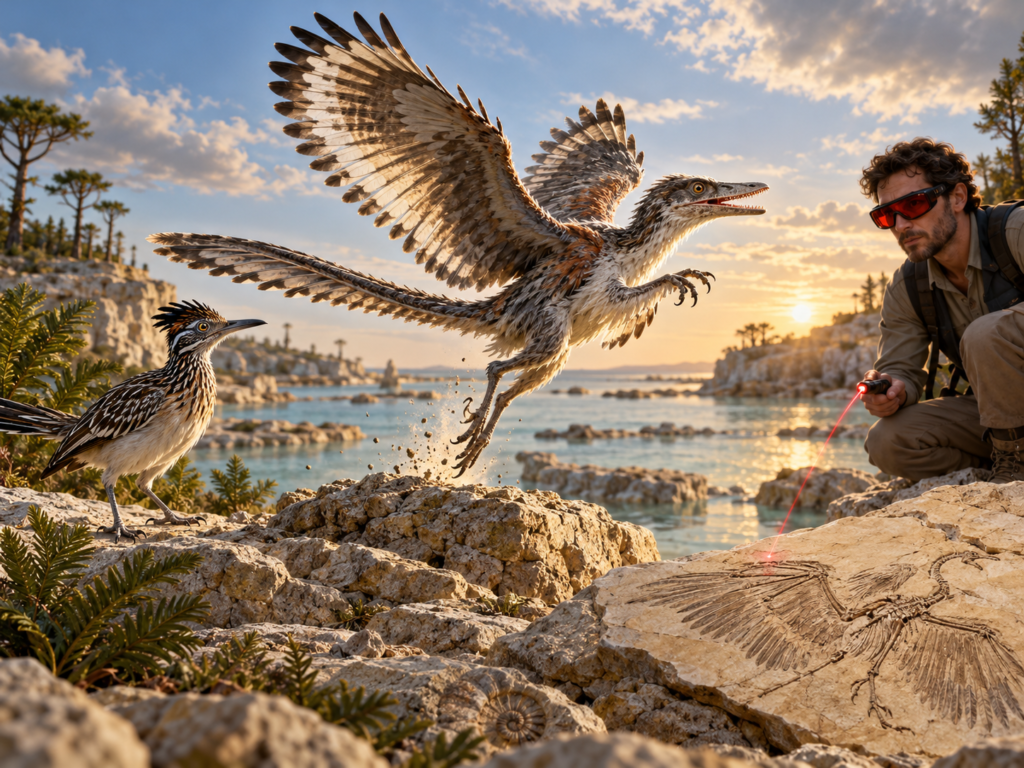
The principle is elegant. The fossil surface is illuminated with a laser of a particular wavelength. Different minerals and chemical residues then fluoresce with different intensities, while a camera records signals that the human eye cannot detect under normal illumination.
The resulting image is not literally a photograph of the original soft tissue. It is better understood as a kind of chemical and structural map of the fossil surface, capable of revealing the boundaries of former biological structures even where their anatomical form has long since disappeared.
At that point, my engineering instinct asks an obvious question: how many old fossils in museum collections contain information we have already found, but have not yet learned how to see?
The answer is probably: a great many. Major paleontological discoveries do not always have to begin with a new expedition. Sometimes it is enough to ask an old fossil a new question.
A Foot from Which More Than Bone Remained
One elegant example comes from studies of early flying theropods. LSF has been used to investigate soft structures of the foot, including keratinized toe pads and scales, together with the anatomy of joints and claws. Such analyses indicate that Archaeopteryx and related early forms had feet that were, to a significant degree, adapted for movement on the ground.
This further complicates the old debate about the origin of flight. Did flight arise from ancestors that ran on the ground and gradually began using their forelimbs to assist movement and takeoff? Or did they climb trees, glide first, and only later develop powered flight?
Archaeopteryx seems unwilling to fit neatly into either category.
Recent ecological reviews suggest that its hind limbs were well adapted for terrestrial locomotion, while the anatomy of the toes indicates some capacity for grasping branches. The hands retained the grasping abilities of their ancestors, which may have helped with climbing. At the same time, large wings with asymmetric flight feathers formed genuine aerodynamic surfaces.
What emerges, then, is an animal that probably moved well on the ground, could climb vegetation and reach higher positions, and was already capable of active movement through the air. It was not a modern bird, but neither was it a passive glider comparable to a flying squirrel. It was an animal with its own combination of biomechanical solutions, some of which no longer exist today.
How Did Archaeopteryx Actually Fly?
The feathers of Archaeopteryx show clear aerodynamic properties. The asymmetry of the primary flight feathers, the size of the wings, and well-developed tertial feathers all strongly indicate the ability to fly.
But its shoulder girdle, thorax, and forelimb skeleton were not the same as those of modern birds. Today’s birds possess a highly sophisticated system that enables powerful wingbeats, precise control of wing rotation and position, maneuvering at low speeds, and efficient takeoff and landing. In Archaeopteryx, some elements of that system had not yet developed into their modern form. The anatomy of the shoulder girdle, humerus, and wrist suggests a different range of wing motion and probably a different flapping mechanism.
So perhaps the question is no longer: Could Archaeopteryx fly?
Increasing evidence suggests that it could.
The more interesting question is: What did flight look like in an animal whose powered-flight apparatus still differed from everything we see in living birds?
It may have used shorter episodes of powered flight combined with running, climbing, and exploitation of wind. It has even been proposed that coastal winds in the Solnhofen archipelago could have helped with takeoff. This is no longer a story about a “primitive bird” that simply had not yet learned to fly well enough, but about a lost biomechanics of flight representing a distinct evolutionary strategy.
Life Between Ground, Vegetation, and Air
Let us now try to return Archaeopteryx from the museum display case to its original world. On the islands of the Solnhofen archipelago, the climate was warm and seasonal. After rainfall, new food resources appeared, insect activity increased, and the availability of small prey changed, while dry periods brought significantly different conditions.
We still do not know the precise diet of Archaeopteryx, but some features of the skull point to good sensitivity in the front of the snout and an ability to manipulate small food items. It is therefore reasonable to suppose that it was an adaptable omnivore, taking small, energy-rich food sources, probably from both animal and plant origin.
It also had to deal with predators. Small predatory theropods such as Compsognathus and Juravenator lived in the wider ecosystem, and younger Archaeopteryx individuals in particular may have become prey. There is even a hypothesis that the fossils found in lagoon sediments may disproportionately represent young and less experienced individuals that were carried out over water by storms.
What we see now is no longer merely a feathered skeleton, but an animal moving between the ground, vegetation, and air, searching for food in a changing environment, avoiding predators, and using a combination of abilities unlike that of any living bird in exactly the same form.
Evolution as a Network of (Im)Possibilities, Not a Chain of Destined Links
Older depictions of bird evolution often presented a neat sequence: a small dinosaur acquires feathers, the feathers become longer, the forelimb becomes a wing, the animal begins to fly, and eventually a bird appears.
Real evolution is far more complex.
Feathers appeared before flight. Different lineages of small theropods developed aerodynamic surfaces of different sizes and probably different functions. Some likely relied more on the ground, others on vegetation and elevated positions, while in some lineages powered flight became increasingly important. Not all lineages moved toward the same outcome, because evolution has no predetermined final goal.
Instead of a chain of preordained links, we see a network of possibilities in which different organisms respond to different ecological challenges through combinations of old and new traits.
Some Birds Never Took Off
A particularly interesting contrast comes from a newly described bird of the Late Jurassic from China, Yuezhuornis yangyuanensis, approximately 150 million years old and therefore from roughly the same time window as Archaeopteryx.
Its anatomy tells a very different story. It had extremely short forelimbs and features indicating a strongly terrestrial lifestyle. The authors of its description interpret it as a flightless early avialan, showing that even very early birds were already occupying different ecological pathways.
It should not be declared an ancestor of modern ostriches, emus, or roadrunners, because there is no phylogenetic basis for that. But the parallel is amusing: while Archaeopteryx was experimenting with wings and air, another roughly contemporary early bird lineage was already showing that wings were not the only possible evolutionary direction.
There were no mammals like Wile E. Coyote chasing these ancestors of the Road Runner 😄, but there was certainly no shortage of predators.
Behind the joke lies a serious evolutionary message: even in the earliest stages of avian evolution, there was never a single path toward modern flight.
So What Was Archaeopteryx?
Archaeopteryx was not “half dinosaur, half bird.” Such a phrase conceals more than it explains. Nor was it simply one link in a chain leading from dinosaurs to pigeons.
It was much more interesting than that.
It represents an early combination of traits that evolution would later redistribute differently. It had a long bony tail, teeth, and functional clawed fingers, but at the same time also possessed developed feathers and aerodynamic wings. It moved well on the ground, probably climbed and used branches, and could also fly in a way that has no true modern equivalent.
This is what we call mosaic evolution: different systems within one organism do not change at the same rate and do not have to become “modern” simultaneously. An old trait can persist beside a completely new innovation, while a new trait does not have to appear immediately in the form it will take tens of millions of years later.
When New Technology Reopens Old Cases
The first known Archaeopteryx fossils were discovered at a time when X-ray CT, digital image processing, sophisticated chemical mapping, and laser-stimulated fluorescence did not exist. The fossils, however, were there all along, carrying chemical traces of structures that once represented skin, keratinized pads, feathers, or other soft tissues.
Researchers of earlier generations could look at them without yet being able to see them.
Today we examine those same fossils again with techniques capable of revealing information hidden in the stone. A laser does not change the past; it changes only our ability to read it.
That has implications far beyond Archaeopteryx. Museum collections around the world contain millions of fossils collected over the past two centuries, many of them studied with methods that are now outdated. The next major paleontological discovery may therefore not come from a new fossil site. It may already have been lying in a museum drawer for decades.
The Theory of Evolution Continues to Evolve After Darwin
Darwin could not have known about genes. He knew nothing about DNA, horizontal gene transfer, retroviruses embedded in genomes, epigenetic regulation, pseudogenes, evo-devo, large-scale genomic analyses, or chemical traces of soft tissues in fossils 150 million years old.
Yet the basic idea of population change through inheritance, variation, and natural selection did not disappear because of that.
What disappeared was the overly simple picture of evolution.
Instead of ladders, we see branching. Instead of finely modified links in a single chain, we see complex biological experiments that represented responses to changing ecological challenges. Some of those experiments opened new developmental directions, others persisted for millions of years, and still others disappeared completely, leaving behind combinations of traits that no longer exist today.
Archaeopteryx has not lost its place in that story. Its story has simply become much richer.
More than a century and a half ago, it showed us that dinosaurs and birds were connected far more deeply than could then be imagined. Today, the same fossils pose a more complex question: what does it look like when life begins to conquer a new physical dimension?
The answer was probably not one perfect flap of a wing. It was a long period of anatomical experimentation in which running, climbing, gliding, and increasingly capable powered flight were combined, while other early bird lineages followed entirely different paths.
One of those experiments left the imprint of its feathers in the stone of Solnhofen. One hundred and fifty million years later, we illuminate it again with a laser and discover that the story of the first flights is still not finished.
Leave a Reply